11. Life History Evolution
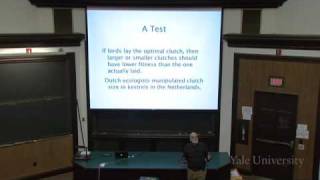
Life-history evolution explains how organisms' size, lifespan, and reproductive strategies result from ecological pressures and internal trade-offs. A Dutch kestrel experiment showed intermediate clutch sizes maximize reproductive success because larger broods increase parental death. Selection pressure weakens with age, which helps explain why aging evolved despite being costly.
Chapters
Okay. Today we're going to talk about life history evolution. And life history evolution deals with some big questions. It's explained why organisms are small or large, why they mature early or late, why they have few or many offspring, and why they have a short or a long life. Basically, what life history evolution does is it analyzes the evolution of all of the components of fitness, all the different things that combine to result in lifetime reproductive of success. And in so doing, it visualizes the design of the organism as an evolutionary solution to an ecological problem. So it's fundamentally about the interface between evolution and ecology. And it is one of the places where scientists confronted the problem of how do we explain phenotypic evolution rather than genetic evolution. So, This is really about the design of the large-scale features of organisms. And it brings us to ask questions about ourselves as well, of course. Why is it that we have a lifespan of about 80 years? Why is it that we're about 3 kilos when we're born, et cetera? Okay, so we fit into this matrix of questions. Now here are a few world records. Biggest baby is a blue whale. 12 tons. And the interesting thing about it is that it will grow to be 60 tons in the next 6 months. So it's really pumping it in. And by the way, a mother blue whale— and most whale mothers actually have muscles in their breasts so that they actively pump the milk into their offspring. Baby isn't just sucking. Baby's attached to a fire hose. Okay? And— And look at what happens to the mom. She goes to warm tropical waters to give birth, has her baby, and then she nourishes that child until it is independent without eating herself. Imagine how big she is, because he turns into something 60 tons. And you can imagine how cranky she is before she swims back to Antarctica to get lunch. Then if you ask yourself, for a given body weight, what is the biggest thing? It's not the blue whale baby, it's the babies, the twin babies of a bat are the largest weight of any offspring in mammals. And she actually flies with them. And in the kiwi, it has a 400-gram egg. If you take a radiograph, if you put a kiwi in a into an X-ray machine, take a radiograph of it. You are to imagine an egg that's occupying about two-thirds of the body cavity. The kiwi, it's got a giant egg. The fewest offspring per lifetime of anything that's out there bearing a significant risk, and this is actually less than humans, is the Mexican dung beetle, that only has 4 to 5 babies per lifetime. Which is pretty remarkable when you think about how risky you would think life would be for a Mexican dung beetle. I mean, how can it get away with only having 4 or 5 babies if some of them are likely to die? But in fact, it has such good parental care that it's around and it's doing just fine, thank you, with only 4 to 5 babies. And the most offspring per reproductive event is orchids. Orchids produce typically billions of seeds. And they are extremely tiny. And the only reason that they can hatch is that they have a fungal midwife that helps them. Orchid hatching is dependent upon fungi. So the mother doesn't have to put the nutrients into the seed. So she makes billions of tiny seeds. And in bivalves and codfish, they can get up to hundreds of millions of eggs per reproductive attempt. So you can see that just by comparing some numbers and looking broadly— and this is a typical thing that happens in comparative biology, it's one of the neat things about it— if you look across the tree of life and you see how different things live their life histories, you immediately start to ask questions. You guys have all been generating wonderful questions this week. You look at that stuff and you say, "Well, why are things big and small? Why do they have few babies or many babies? What has caused the evolution of all of this diversity?" So here is the largest whale and the smallest dolphin. So this is the whale radiation. You can see that since the ancestor, there's been considerable change in body size. Here's Pipistrellus flying with babies. Here's a dung beetle, and it's going to lay its egg into that pile of dung. That's why it's going to have an extremely well-protected baby. Not too many things are going to come along and eat baby. And here's a kiwi with its egg. Okay? So diversity. So in the history of ideas, life history theory and the rest of evolutionary and behavioral ecology fit about here. Darwin showed us that natural selection and descent with modification from ancestors can explain a lot, but then genetics remained a problem until 1900. Then we had the genetical reaction to that issue, which is the Neo-Darwinian synthesis that basically says Darwin works with genetics. And this concentration on genetics then, in its own turn, elicited a reaction. So this is a reaction to that, And "What's the role of phenotypes in evolution?" is the reaction to the neo-Darwinian synthesis. So the phenotypic reaction, which has been going on for about 40 years, it has a selectionist part, that is, how are phenotypes designed for reproductive success? And it has a developmental part. What are the restrictions on the expression of genetic variation? So the phenotypes are actually both being designed, by natural selection for reproductive success, and in the process of their production, they are themselves editing genetic variation. So life history evolution is the part that explains the design of phenotypes for reproductive success. And it concentrates on size at birth, how fast things grow, age and size at maturity, reproductive investment, and mortality rates and lifespan. So part of life history evolution is, why do we grow old and die? And after a lot of discussion, it was possible— this is after about 20 years of discussion— to make this simple statement. What causes life histories to evolve? They result from the interaction of extrinsic and intrinsic factors. So the extrinsic factors are are things that are influencing the age-specific rates of mortality and reproduction. And that's where ecology comes in. It's not just ecology. There's a lot of phylogenetic effect on this stuff. But the point is that if you look at whatever is affecting changes in mortality and reproduction, in age and size of the organism, you will be able to explain a great deal of what you see in the life history. But that's not enough. There's an interaction between that and factors that are intrinsic to the organism. And the intrinsic factors are conceptualized as tradeoffs among traits. The idea here is there's no free lunch. If you change one thing in evolution, a byproduct of that change will be a change in another trait. So even though that you are gaining fitness through changes in one trait, almost inevitably whatever you change is going to cause a decrease in fitness in some other trait. And this forces compromises. So the intrinsic factors then can be looked into, and we find phylogenetic effects, developmental effects, genetic effects, physiological effects, all sorts of things. Tradeoffs in an evolutionary situation are often conceptualized as being strictly energetic. If I take calories away from my growth in order to reproduce and make more babies, then I won't be so big next year and I can't have so many babies next year. That would be kind of a standard physi— physiological story about a trade-off. But they can also occur in many other ways. So that would be a physiological story, but certainly there are developmental and genetic influences on trade-offs as well. So there's a lot of biology that's hiding behind these simple summary statements on this slide. In the rest of the lecture, I'm just going to show you how to explain agent size at maturity, reproductive investment, and aging and death. So not too much. This is kind of a standard statement out of life history theory. And this generic statement could be applied to clutch size and lifespan and a lot of other things. But let's just look at age and size at maturity. They will be optimal when the positive difference between the benefits and the costs— so the difference between the benefits and the costs— is maximized. And we can conceive of that as either being maximized just at a stable equilibrium point. That's kind of a simple statement. That's a theoretical statement. So that would be, okay, everybody in this species, they ought to mature at just one age and size, which is a little unrealistic. Or we can use that kind of analysis to predict a stable equilibrium reaction norm. So here we're beginning to use this idea that we got of a reaction norm. And that one summarizes pretty easily. You're going to, you know, whatever problem you're faced with, you're going to mature at the age and size where the payoff in fitness is going to be greatest. The problem, analytically, is to decide what you have to bring into the mix in order to successfully make that prediction. You want to keep it as simple as possible, because it can get very complex, but you want to keep it realistic enough to actually be successful. So it's a balancing act. Now, with— I'm going to show you one way to do this. If we make four general assumptions, we can predict age and size at maturity. Here they are. The first one is that if you're older when you first reproduce, your offspring are going to have better survival rates. They will be of higher quality. So one reason to wait is that you get higher quality offspring. Another reason to wait is that because you've been growing for longer, you've taken longer to grow before you start to reproduce, you can have more of them. Because you're bigger. Especially important in plants and in fish. However, these advantages of delaying maturity are counterbalanced by the advantages of having a shorter generation time, and you can only get a shorter generation time if you mature earlier. Let me just illustrate the advantage of a shorter generation time. I give you $100 and I tell you you can invest it in the bank that's going to give you compound interest once a day, On the one hand, or once a year on the other hand. You all know the advantages of compound interest. You get interest on your interest. Right? A shorter generation time is the bank that gives you interest earlier. You get grandchildren quicker. Okay? So that is basically the elements that you need to put into a quantitative tradeoff. Delaying, you can get higher quality or more offspring. Doing it quicker, you're going to get a shorter generation time and a quicker payoff. Now, in a population that's at evolutionary equilibrium, these advantages and disadvantages should have come into balance. So let's see how that might work. Here's a simple example. This is using data from the Western fence lizard. And what you're looking at here, this plot here, where you see these curves going up and down, that's a fitness profile. So we have some kind of trait along the y-axis. In this case, it's age of maturity along the x-axis. Along the y-axis, we have relative fitness. So this is the rate at which a population of organisms with that age of maturity would grow, given what we know about the physiology and mortality rates of fence lizards. And if we just put in one of those assumptions, which is that the bigger they are, the more babies they have. So their fecundity grows linearly with size. Their optimal age of maturity is just about 12 months. If we put in that if they get higher quality offspring as they delay maturity, given the assumptions in the model, we predict actually that they ought to be maturing at about 6 months. Their observed age at maturity is 10 months. That indicates that this effect is probably important and perhaps accurately modeled. This number tells us that, well, perhaps we don't really understand what makes for a good baby lizard. Okay? And you can see that, interestingly, the age at maturity is pretty strongly peaked. I mean, the fitness profile has a peak that's pretty close to one value. That means there's pretty strong selection operating on this. It's not flat. Now, if you repeat that kind of thing— and by the way, there's a bunch of math behind that. I'm just waving my hands and covering up that black box. If you repeat that for a bunch of fish species that are growing in different kinds of conditions— these are haplochromine cichlids in Lake Victoria. The painted greenling lives in Seattle. These roaches are living in Greece. And these are all cases in which very good population biology has been done for long periods of time in the field, so we know growth rates and mortality rates, and we have some estimate of tradeoffs. Then that kind of thinking says, this is the predicted age at maturity, and this is the observed age at maturity, and the correlation is 0.93. So it looks like that way of thinking is capturing something that is is not a bad reflection of what's going on in nature. This sort of result doesn't mean you've got the right answer. You can have the right answer for the wrong reason, because this is just descriptive work. This is not a manipulative experimental study. We'll see such an experimental study later on. However, that's not the whole story. I now want to extend that to the case when growth rates vary. And I want to introduce you to the idea that age and size at maturity can have a reaction norm. And the way I want to do that is by dealing with some incredibly blockheaded strategies. Okay? So here we have rapid growth. So this is an organism that is born down here, and it's well-fed, and it grows rapidly, so it gains weight. Well, reaches a large size. And this is an organism that grows slowly. It's under food restriction down here. Now let's take the blue strategy. This is a very, very simple one. And what it says is, I'm always going to mature at the same weight. If that organism is growing rapidly, it matures at a pretty early age. But if it's growing slowly and it adheres to this rule, it has to wait a long time until it matures. And its problem here is that it might die before it matures. So that strategy has the cost of mortality. On the other hand, if it's always the same age when it matures, under good circumstances it's doing okay. But under poor circumstances it's much smaller, and therefore it can have fewer babies. And so the problem here is fecundity. It's going to not have as many babies if it does that. And so just intuitively you might think that there is some kind of intermediate compromise, so that when it is not being fed as much, it changes both its age at maturity and its size at maturity. And in fact, this kind of thing can be calculated. This is an optimal reaction norm for agent size and maturity. They don't all look like this, OK? This is a common one, but there are conditions under which you can make this thing bend. You can actually sometimes get them so that they go up like this, under very special circumstances. It depends on a bunch of stuff. I don't want to trouble you with the complexities. I just want you to take home the message that you can predict what the plastic flexible response should be if evolution has come to equilibrium. And for this one, basically what this graph is telling you is this. This is the reaction norm here. These are growth curves here. So this is good, good conditions. This is poor conditions. And what this picture is telling you is that when life is good, You should mature when you are young and big. And when life is bad, you should mature when you're old and small. Okay? That's the English take-home message out of that picture. Well, when Nile perch were introduced to Lake Victoria, there hadn't been any Nile perch in there before. And they went bananas and ate their way around the lake. And in the process, by the way, they probably drove about 200 haplochromine species to extinction. But while they were going through their initial population burst, and they had a lot of food, they were about 6 feet long. This is the business end of a Nile perch. You can see it's a big fish. After they had expanded in the lake, which occurred between 1976 and 1979, they ate down the population of their prey. They— there wasn't as much food, and they didn't grow as well. And they slid down this reaction norm. And now, instead of being 6 feet long, the Nile perch in Lake Victoria are about that big. They still form a fishery and people are still making money on selling Nile perch fillets, but they're much smaller. And that was a predictable thing. Okay? And this will happen whenever population densities change. Back in the 1930s, 1940s, and 1940s, there was a huge sardine fishery off the coast of California. John Steinbeck wrote novels about it, short stories. There's a book called Cannery Row that talks about the Monterey Bay sardine canneries. In the 1950s, that fishery collapsed, not because of overfishing, but because of changes in the oceanic conditions where the baby fish were growing up. At the time that it collapsed, there were sardines that had been born under better conditions and started to grow. And then all the competition went away. Nobody else came along, because all the baby sardines were getting killed by bad conditions out in the ocean. Just before the fishery folded and there were no longer enough sardines to catch, the fishermen in Monterey were catching female sardines that were 1 meter long. So they had gone in the other direction. They'd gone up the reaction norm. These things are predictable as population density changes. I'd like to give you one more example. And it has to do with the issue of whether or not the mammals died out because of bad weather or overhunting. Dan Fisher, who's a paleontologist at the University of Michigan, has recovered a lot of mammoth bones from a Native American mammoth slaughterhouse that was outside of Ann Arbor. They used to kill the mammoths and then store them under ice in a lake over the winter so that the other predators wouldn't get the meat. And there are a lot of mammoth bones very close to Ann Arbor. And you can ask yourself, when you look at a mammoth bone, you can tell how big the mammoth was and whether or not it is mature, because the bones of all mammals undergo a change when they reach maturity. Now, if it was bad weather, then they would have been growing slowly and they should have been small and older when they matured, according to the reaction norm. If it was hunting, then just like the California sardine, When the population density drops, each individual has more to eat and they should have been big and young when they matured. Do you think they were old and small or big and young? How many for old and small? Bad weather? A few. How many for young and large? Hunting? Most people believe the overkill hypothesis. Yeah. They were young and large. And some of them had arrow points embedded in their ribs. So you can use that for various things. This is what that model tells us about human females. These are some pretty theoretical growth curves for human females under poor conditions and under good conditions. We actually have data on how female age and size at maturity has changed. There are measurements on women working in industrial squalor in North England in the 19th century. And there are good records measured on Hutterite colonies in North America in the 20th century. The 19th century women were poorly nourished. The 20th century women were well nourished. They moved right up a reaction norm. They got younger and bigger when they matured. And it was about 4 years difference. So they went— there are various measures of when a woman is mature, physiological measures, but they kind of all move together. So it's about a 4-year advance, earlier maturity in the 20th century. And this other line here illustrates another point that I want you to take away from this. If modern medicine were to keep juvenile mortality rates, as low as it currently does, then it would cause a further shift in age of maturity in humans. And that shift is represented here. This probably would take somewhere around 5,000 or 10,000 years to occur. This is the evolutionary genetic response. This is the immediate developmental response to better nutrition, and this is the evolutionary genetic response to a drop in juvenile mortality rates. The whole reaction norm evolves. It will move up and down. It is embodying an evolutionary set of rules of thumb, okay? Contingent decisions. If I'm well nourished, do this. If I'm poorly nourished, do that. And those things evolve. Okay. Now the second major life history trait is, once you've matured, How many babies should you have, and how big should they be? You want to be an orchid with billions of tiny ones, or you want to be a kiwi with one big one? Well, the ideas on this go back to David Lack. David Lack was the man who more or less created the idea of Darwin's finches in the Galápagos. Darwin's finches, as a concept, emerged in the middle 20th century. They were never called Darwin's finches before David Lack went to the Galápagos, studied them, came back and wrote a book called Darwin's Finches. It was 100 years after Darwin had— 120 years after Darwin had been there. And he went on to become head of the Edward Grey Institute at Oxford, which is an ornithological institute and one of the best places in the world to go if you're interested in bird biology. And you're not working with Rick Prum at Yale. So what David said basically was this: if nestling survival decreases as clutch size increases, then an intermediate number of eggs produces the most fledglings. The idea behind that was this: if you make too many babies, you won't be able to feed 'em. There are only so many hours in the day. You might be able to work as hard as possible and not bring off a clutch of, say, 10 babies, but you could do quite well with 5. Now I'm going to show you that he was wrong on the details, but he got the main point, which is that fitness is often maximized at intermediate reproductive investments, particularly in organisms that reproduce more than once per lifetime. You don't do it all now. You hold some back, and you actually do better if you spread it out. So if we then take Lack's idea and we make a simple model out of it, basically what he was saying is this. As clutch size goes up, well, that just means that eggs go up. But if survival goes down as eggs go up— this is the per-egg survival probability— basically this is saying that if you only laid 1 egg, you'd have very good survival, and if you lay 10 eggs, they all die. You can turn that into an equation for how many fledglings do you get for a given number of eggs. Well, it's going to be 1 minus a constant times the number of eggs you lay. Which means, if you multiply that out, that you've got a quadratic term here in eggs, and that is what leads to the parabola. It's this quadratic term. Quadratic term. That means that as clutch size goes up, the number of babies that you get out of it has a parabolic form with an intermediate optimum. And you then just do the standard basic calculus thing of taking the first derivative, setting it equal to zero. It tells you that this point right here is going to be at 1 over 2c in this equation. And if c is 0.1, this optimal number of eggs will be 5. And the number of fledglings that you get out of it will be 2.5. Of course, you never get 2.5, but that's just because the model's continuous and the eggs are discontinuous. Well, if this is the case, if birds are laying the optimal clutch, then a larger or a smaller clutch should have lower fitness. Basically, all we're saying is that if we were able to take a bird And she wants to do this, but we give her either fewer eggs or we give her more eggs, then she should have lower fitness. This should be the best, which she naturally does, and if we perturb that, she should have less fitness. This was done on kestrels in the Netherlands by Dutch ecologists in a rather remarkable study. A kestrel is a sparrowhawk. And these animals live— these birds live for several years. And the Dutch ecologist actually followed them long enough to count the grandchildren. So he went 3 generations. So this is the setup. They reduced the size of 28 clutches, enlarged the size of 20 clutches, and in 54 clutches they took the eggs out and put them back again. Those are the controls. And if you just look at this, it looks like these birds should be laying more eggs. Because if you look over at the enlarged clutches, they've been able to change the brood size up by 2.5. They've been able to get more fledglings out. They've gotten nearly 2 more fledglings out of the enlarged clutches. And the reproductive value of that clutch, which is how many grandchildren do I get out of that clutch is higher. So it looks like these birds are blockheaded. They should be laying more eggs. But that's only looking at what happens that season. While they were examining these birds, one of them, Sergej Dan, is a good physiologist, and so he did an experiment with doubly labeled water. He wanted to find out how hard the birds would work. And they were coming into nest boxes. So mommy and daddy kestrel fly into nest box with food for baby. Evil Dutch ecologist sitting in back of nest box takes food away from baby. Baby cries. Baby gets hungry. Mommy and daddy work harder. Evil Dutch ecologist takes away food. Mommy and daddy work even harder. How hard do mommy and daddy work? Mommy and daddy work about 8 hours that day. Daylight's about 16 hours a day in the summer in North Holland. And they hit a rate of— physiological output, which is nearly 4 times basal metabolic rate, which is what Lance Armstrong puts out on the Alpe d'Huez in the middle of the Tour de France. So the Dutch ecologists basically forced these birds to work as hard as a peak human athlete would, and then they quit after 8 hours, because they didn't want to die. And then the Dutch ecologists gave the babies their food. Just so you don't have nightmares about that. Okay? So that introduces parental survival. If you increase the clutch size, the parents died the next winter at a higher rate, because they worked harder. Okay? And if you add all of that up, the residual reproductive value of the rest of their lifetime, The number of grandchildren they would get out of the rest of their lifetime was highest for the reduced broods, intermediate for the control broods, and strikingly lower for the enlarged broods because of this effect. If you die before the next year, you get zero babies next year. So if you look at their total reproductive value, which is the value they got this year plus the value they got in the rest of their life, it's highest for the control group. And if their clutches were enlarged, they had one grandchild less. And if their clutches were reduced, they had half a grandchild less. Which has an interesting take-home message. These Dutch kestrels know what's best for them. They lay the right number of eggs. That's the control group. So the take-home points basically are that what's going on here is the clutch size is trading off with with an important fitness component, but it's not fledgling survival. Okay? It's parental survival. In this case— I mean, it's different in other species— but in this case, the reason that they don't lay more eggs is that they themselves are more likely to die, not that their offspring are more likely to die. And these kestrels are optimizing their reproductive investment with a clutch that's of intermediate size. They could lay more eggs, but they don't. They know how many to lay. Okay, so that's just one example of clutch size analysis. It's a big literature. There's a lot of experiments on this. Now let's go to lifespan. So I'm taking you through the major life history traits from birth to reproduction to death. In Fragment of an Agon, T.S. Eliot wrote, "Birth, reproduction, and death. That's all the facts when you come to brass tacks. Birth and reproduction and death." He wrote that in the 1930s, I think. I didn't realize that T.S. Eliot was a behavioral ecologist. Evidently he was. So reproductive lifespan, under this kind of analysis, is a balance between selection that increases the number of reproductive events per life—you live longer, you can reproduce more—and effects that increase the intrinsic sources of mortality with age. And it's this idea that there is an evolution of aging or of senescence, there's an evolution of the body falling apart as a byproduct of something, which is the key feature of this part of life history theory. So the first kinds of selection pressures are going to lengthen life to give you more reproductive opportunities. But if there are byproducts that are causing intrinsic increases in mortality rate, those will shorten your lifespan. So these things then come into some kind of balance. Any increase in intrinsic mortality rates or decrease in reproductive rates with age is called aging or senescence. So now we're talking about why people fall apart when they get old and why organisms age and die. To do that, I need to introduce you first to the way selection operates at different ages. Selection is quite age-specific in its impact. Any selection pressure that lengthens life is going to be one that decreases the relative contribution to fitness of offspring and increases that of adults. So if an adult has survived, to some intermediate age, and juvenile mortality in that species is pretty high, then the adult represents a relatively improbable event that's quite valuable. And if it's making babies in that environment, each of them has a relatively low chance of surviving to be that big and that old. And therefore, there is a certain fitness advantage in investing in the preservation of that adult. Because it's unlikely that you'll get another one up to that state. The things that will do this are lower adult mortality rates and higher juvenile mortality rates. So if life is relatively good for adults and pretty risky for juveniles, then— and infants— then you're going to get the evolution of a longer lifespan. But in contrast, if adult mortality rates increase, then organisms should evolve more rapid aging, basically because there really isn't much point in maintaining a body baby that's going to be dead anyway for other reasons. Why should I take away from my reproduction and invest it in, say, disease resistance or running away from predators if I'm not going to be able to avoid them anyway? Then I should make more babies. Okay? So those are the basic ideas. And I'd like to illustrate a little bit of the math behind this with a pictorial model. So this is why senescence evolves. I'm going to use the fruit fly, Drosophila, as the model organism. We're going to start this thing off not when it's an egg, but when it ecloses and is an adult. And we're going to say that our model has no intrinsic mortality at all. So this one doesn't age. This is our baseline. This is what happens if an organism doesn't age. Its risk of dying is 20% per day. And every day it lays 10 eggs. Okay? So on the first day it gets 10 eggs. On the second day, 80% of them are still around and each of them lays 10 eggs. And on the third day, 64% of the original are still around, 0.8 times 0.8, 10 eggs, ta-da-da-da. And this thing is potentially immortal. Okay? So it can just go on pumping out the eggs, if it survives, for as long as ever. And its probability of survival isn't changing with age. It's 80% each time. This one gets 50 progeny. We do that just by using an infinite series. Okay? And the numbers were set up to give you a nice simple output. Okay? The numbers are cooked. So this one gets 50. Now, what happens if everybody dies between the 19th and the 20th day? That one gets 49.3. That's all the difference that death at old age makes. And this is in a case where there's no senescence, right? This is kind of like light bulbs failing or something like that. However, now let's throw in a little life history trade-off. And it's a really small one. This genotype here, because it can lay 11 instead of 10 eggs, on the first day of life dies between the 19th and the 20th day. It leaves 50.3 progeny. It has a 0.6% fitness advantage. If we introduce this genotype into the populations of the ones that live forever, it will take over. There won't be any immortal flies anymore. There will be flies that have evolved a shorter lifespan because they had a reproductive advantage early in life, and it didn't It didn't take much of one to do it. As you contemplate your own mortality, I hope you realize that the Drosophila example, in fact, is non-trivial. It's giving you an important message. This is the strength of selection on further survival in human males in the United States in the year 1960. Calculated from real demographic data from the U.S. Census. This is the partial derivative of fitness with respect to further survival. And it's a very interesting picture. What it shows you is that you— as soon as you become a teenager and you have some probability of surviving in that human population, your fitness starts to drop, because as soon as you've had a baby, you have some probability of grandchildren. And it shows you that after the age of 46, evolution doesn't care if you're there anymore, from the point of view of getting grandchildren. As someone who is out here, I would like to congratulate all of you. There's a reason I look different from you. Now, this way of looking at aging basically says that aging is a byproduct of selection for reproductive performance. And the reason that it occurs is that there's an accumulation of a lot of genes. And they have positive or neutral effects on fitness components early in life, and they have negative effects on fitness components late in life. The positive effect is called the— Antagonistic pleiotropy hypothesis, the idea is that the gene has two effects, good early and bad late. It's like that one that gave the fly one more baby on the first day of life, but killed it off at the 19th day of life. And neutral effects early and negative effects late is called the mutation accumulation hypothesis. And these two hypotheses formed sort of the intellectual basis of research on the evolution of aging for quite a while. And they turn out to be not too productive. It looks like, in fact, most of the cases that have been well investigated suggest that it's positive effects early and negative effects late, not neutral early and negative late. Okay? But it's hard to distinguish between these sometimes. A general take-home point is this, that organisms age is actually the best evidence we have that it's the replication of genes, not the survival of organisms, that is the ultimate the object of evolution. So that gives you strong empirical evidence that a gene-centered view of evolution is, in fact, empirically correct. This is extremely discouraging for the organisms that have consciousness and the ability to analyze the situation. So a bit of experimental evidence. By the way, there have been— We did 5 or 6 experiments like this. I'm just showing you because this is the one I did. We had 2 treatments. We had high and low adult mortality. And if you followed the logic so far, then you already know that the— if you apply high adult mortality, then the organism should age rapidly. And if you apply low adult mortality, they should evolve to age more slowly. So if you make the environment risky, why try to invest in surviving, because somebody's going to kill you anyway? In which, in this case, it was a Swiss laboratory technician that was doing the killing. One can imagine that it might have been a lion or something like that. The result is that after 5 years, which is about 70 to 110 generations in these flies, aging evolved as expected. The higher extrinsic mortality rates had produced shorter intrinsic lifespans, and the change was about 5 days. It's convenient that a day in the life of a Drosophila is about a year in the life of a human, so that gives you some feel some kind of intuitive feel for what this means. Basically what that means is that if we had started applying this strength of selection at the time of the Trojan War, we would have produced a response in the human population of about 5 years by now. Okay? Just to put it back into the human time scale. There's a paper here, you can go read about that if you want. It gives you an entry into that literature. To summarize today's lecture, all the major life history traits—age and size of maturity, number and size of offspring, lifespan, reproductive investment—are involved in trade-offs. And that causes them to come to evolutionary equilibrium at intermediate, not at extreme values. They are all under stabilizing selection caused by trade-offs. Age and size at maturity, number of offspring per birth and per lifetime, and lifespan and aging have all evolved. I'll just riff on this for a moment to tell you how you've changed compared to chimpanzees and bonobos. Humans live a bit longer, about, oh, 20 years longer. Humans— the unique human life history traits that appear to have evolved since we shared ancestors with chimpanzees and bonobos are menopause, which does occur, but rarely, in zoo chimps and is almost never observed in the wild. The most striking thing, though, is that we can have babies twice as fast as they can. The average time in a Neolithic or hunter-gatherer in our society between births is 2 years in humans. And in chimps it's 5 to 6. That, despite the fact that human babies are much more helpless and need a lot more parental care when they're born. So in fact, humans have somehow managed to almost double the reproductive output of chimpanzees. And it appears that they've done it through social interaction. So family members help raise the kids. Sometimes even partners help raise the kids. Grandmothers help raise the kids. But there's a lot of help. And so the reason that the interbirth interval in humans has been shortened dramatically in the last 5 or 6 million years is because we have become a much more highly integrated We have a much better integrated family life. The evolution of all of these traits can be understood, in general, as an interaction between extrinsic ecological conditions that determine mortality rates and conditions inside organisms that cause tradeoffs. So if you're looking for a general explanatory structure, it is that the environment poses problems and when you answer that problem with a solution, you are forced to make compromises. And we know usually which kind of compromises, and we are now in a position to say, if you're looking in the environment, you should look for these kinds of factors. Okay. Next time we're going to extend this framework into a particular part of life history evolution called sex allocation, and how investment is divided between male and female function, and when it pays to switch sex and to be born as one sex and turn into the other.
More from Farzin
Medicine Without Evolution is like Engineering Without Physics- Randolph M. Nesse, MD